We Go Fast,You Go Forward
September 16, 2026
When it comes to engineering T cells for cancer immunotherapy, mRNA-based approaches are gaining serious momentum. Unlike traditional viral vectors, mRNA enables transient expression—CARs are produced for a limited period before being naturally degraded. This built-in safety feature reduces the risk of long-term side effects, reduces the risk of T-cell exhaustion, and even allows for repeated dosing to fine-tune the therapeutic response.
But there’s a catch. For mRNA to work well in T cells, it needs to be efficiently translated into protein. And one of the biggest factors controlling translation efficiency is hiding in plain sight: the 5′ untranslated region (5′ UTR) .
Think of the 5′ UTR as an instruction manual located at the front end of an mRNA molecule. It doesn’t code for protein itself, but it plays a critical role in determining how well the coding sequence gets translated. Most standard mRNA therapeutics use a 5′ UTR derived from the human α-globin gene (HBA1)—it’s stable, well-studied, and works reasonably well in many cell types. However, T cells are unlike most other cell types. They are highly specialized immune cells with unique translational needs, and HBA1 simply isn’t optimized for them.
A team of researchers (Gibor et al.) recently asked a straightforward but powerful question: what if we replace the generic HBA1 5′ UTR with sequences taken from genes that are naturally highly expressed in T cells?
They designed a library of mRNA constructs featuring 5′ UTRs from a range of T cell–relevant genes—cytokines like IFN-γ and TNF, effector molecules, checkpoint receptors, and activation markers. Each construct was otherwise identical, with the same coding sequence, the same 3′ UTR, and the same poly(A) tail. This design allowed the team to isolate the specific contribution of each 5′ UTR to protein expression.
General scheme of mRNA constructs used throughout the research:

All 5’ UTR constructs used in the research:
5’ UTR | Accession number |
Globin (HBA1) | NM_00058 |
IFN-γ | NM_000619 |
TIGIT | NM_173799 |
LAG3 | NM_002286 |
TNF | NM_000594 |
TOX | NM_014729 |
GNZB | NM_004131 |
IL-2 | NM_000586 |
CD3-epsilon | NM_000733 |
CD3-zeta (CD247) | NM_000734 |
CD39 | NM_001776 |
PD1 | NM_005018 |
TIM-3 | NM_032782 |
CD69 | NM_001781 |
The results were striking. Some 5′ UTRs dramatically boosted protein output. The IFN-γ UTR, for instance, nearly doubled luciferase expression in primary human T cells. Others produced the opposite effect: the TNF UTR consistently cut expression by about half. The effect wasn’t subtle, and it wasn’t predictable by simple measures like GC content or predicted RNA stability. In fact, in silico predictions of RNA folding energy showed little correlation with actual expression levels—a reminder that biology doesn’t always behave as predicted.
And here’s an important twist: these differences were unique to T cells. When the same mRNA constructs were tested in HEK293 cells, a standard laboratory cell line, the expression patterns vanished. This finding highlights an important point: these UTRs are not universally enhancing or suppressing translation; they are interacting with T cell–specific machinery in ways we are only beginning to understand.
Building on these findings, the team moved from reporter genes to a clinically relevant payload: a CD19-directed chimeric antigen receptor (CAR). They built CAR-encoding mRNAs using several of the most promising 5′ UTRs and tested them in human T cells.
The TIGIT 5′ UTR emerged as a standout. CAR expression levels with TIGIT were slightly lower than with the standard HBA1 UTR, but functional performance told a different story. When T cells were co-cultured with CD19-positive target cells, the TIGIT UTR drove stronger IFN-γ secretion at low effector-to-target ratios—suggesting greater functional activity per CAR molecule expressed on the cell surface.
Perhaps the most valuable finding came from looking at what happens when CARs are expressed without any target antigen present. This phenomenon, known as tonic signaling, is a well-known challenge in CAR-T biology. When CARs become activated in the absence of antigen, T cells become prematurely exhausted—hey encounter tumor cells.
Here, different 5′ UTRs produced dramatically different outcomes. The HBA1 UTR generated substantial IFN-γ secretion even without antigen, indicating strong tonic signaling. The TIGIT UTR showed similar background activity at baseline. But the TNF UTR was a different story entirely—it kept tonic signaling to a minimum, producing almost no IFN-γ in the absence of target cells.
The team went further, using virus-specific T cells (VSTs) that already express high levels of PD-1—a marker of chronic activation. When these cells received a CAR built with the HBA1 UTR, they rapidly upregulated TIM-3 and became PD-1⁺TIM-3⁺ double-positive, a signature of deeply exhausted cells. By contrast, CARs built with the TIGIT or TNF UTRs did not induce this exhausted phenotype. The cells maintained functionality without developing an exhausted phenotype.
From a clinical development standpoint, this work offers a practical toolkit. Different therapeutic applications may call for different expression profiles. A CAR intended for solid tumor applications with a suppressive microenvironment might benefit from a UTR that supports high and sustained expression. In contrast, a CAR targeting a hematologic malignancy such as B-ALL might perform better with a UTR that balances efficacy against tonic signaling to preserve T cell fitness over the long term.
The TIGIT 5′ UTR appears to strike a particularly attractive balance: moderate expression levels paired with strong functional activity and reduced tonic signaling compared to the standard HBA1 design. For developers working on mRNA-based CAR-T programs, this is exactly the kind of optimization that can make a real difference in the clinic.
The transient nature of mRNA expression—once seen as a limitation—is increasingly viewed as a feature. It provides a built-in safety mechanism, and advances in lipid nanoparticle (LNP) technology are making it possible to deliver mRNA directly to T cells in the body, opening the door to in vivo CAR-T generation. With the right UTR driving expression of the right CAR, we may be able to engineer T cells without ever removing them from the patient.
This study also highlights a broader principle: empirical testing remains essential, even in the era of increasingly sophisticated in silico prediction tools. When it comes to translation control, each UTR–ORF combination needs to be tested experimentally. There’s no shortcut, and no algorithm—at least not yet—that can reliably tell you which UTR will work best for your specific payload in your specific cell type.
At Quintara, we’ve built extensive experience in mRNA-LNP development and are actively applying these insights to in vivo CAR-T programs. Our proprietary 5′ UTR sequences have demonstrated strong expression of both single-target and dual-target CAR constructs in relevant cellular models.
If you’re developing mRNA-based cell therapies—whether for oncology, infectious diseases, or gene-editing medicine—let’s talk. Selecting the right mRNA backbone can have a significant impact on therapeutic performance.
Gibor G, Tzvi N, Meir A, et al. Engineered mRNA backbones for gene expression in human T cells. Molecular Therapy: Nucleic Acids, 2026, 37: 102913. DOI: 10.1016/j.omtn.2026.102913.
We Go Fast, You Go Forward
 sales.us@quintarabio.com
 1-617-789-6111
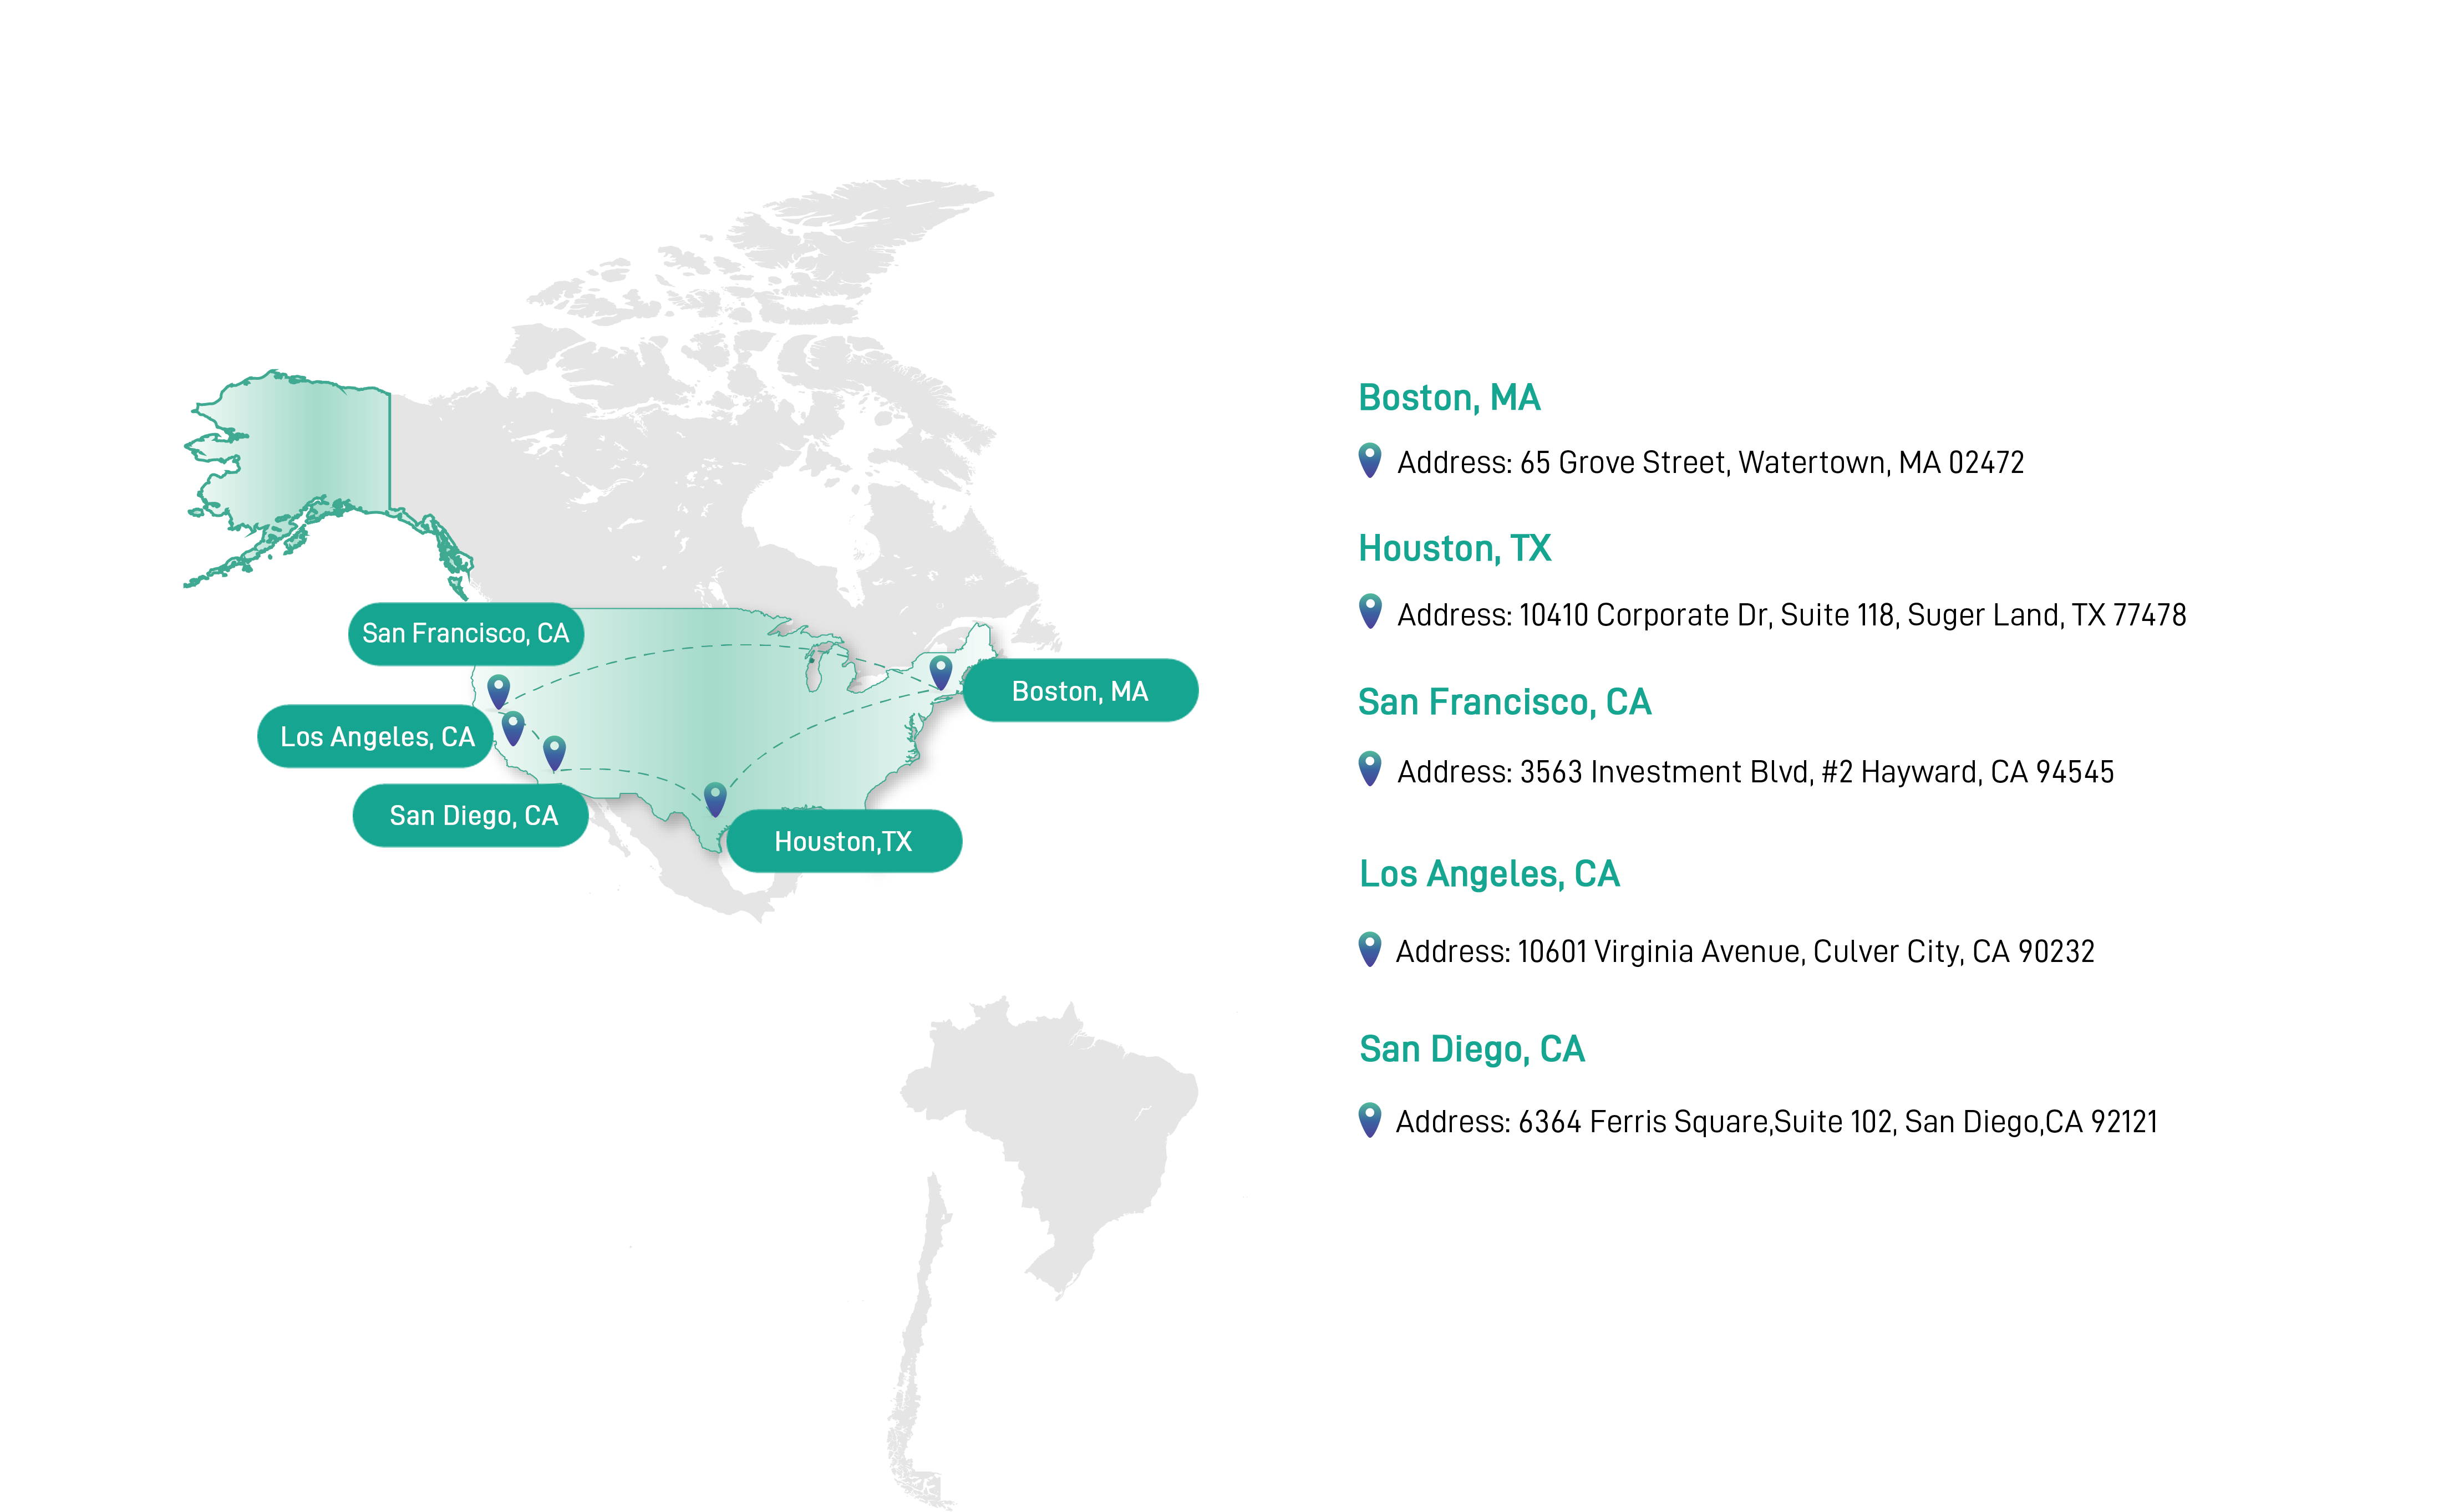
 3563 Investment Blvd, #2, Hayward, CA 94545sales.us@quintarabio.com1-617-789-611165 Grove St, Suite 102, Watertown, MA 02472sales.us@quintarabio.com1-617-789-611110410 Corporate Dr. Suite 118, Sugar Land, TX 77478
sales.us@quintarabio.com
1-424-549-091110601 Virginia Avenue, Culver City, CA 90232sales.us@quintarabio.com1-619-823-08956364 Ferris Square, Suite 102, San Diego, CA 92121Quintara Biosciences © 2025 All Rights Reserved | Site Map | Terms of Use | Privacy Policy


 Login
 Order
 Contact Us
 Contact Us